Microbiome Synergy: Bacteroides and the Science Behind Acemannan’s Benefits
Synopsis: Bacteroides spp. harbor dedicated β-mannan polysaccharide utilization loci (PULs) that integrate surface/endolytic mannanases with accessory esterases and exo-acting hydrolases, enabling efficient degradation of complex acetylated β-mannans from the diet (Reddy et al., 2016; Bågenholm et al., 2019; Déjean et al., 2020). These β-mannan PULs are transcriptionally induced by galactomannan and glucomannan substrates and encode surface-exposed GH26 endo-β-mannanases, periplasmic processing hydrolases, and SusC/D-like transport proteins, providing a complete modular system for capturing and deconstructing high-molecular-weight mannans into fermentable oligosaccharides (Reddy et al., 2016; Bågenholm et al., 2019).
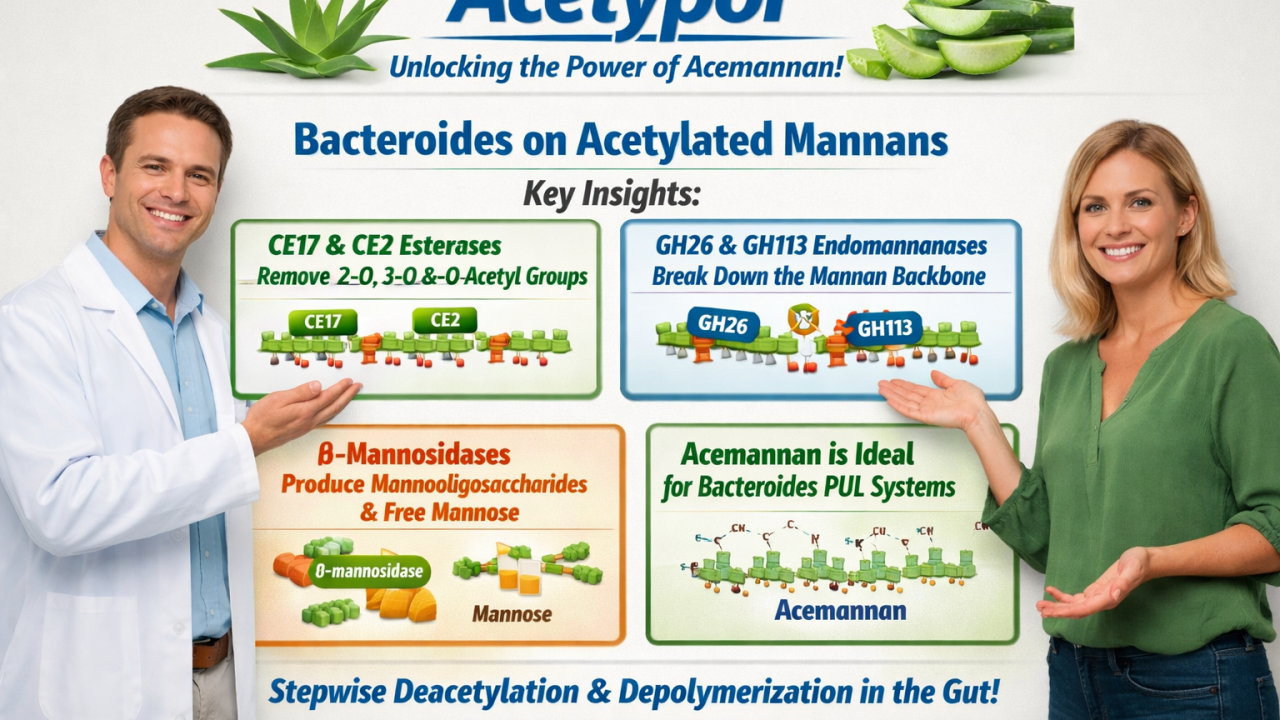
Although detailed biochemical work on acetylmannan deacetylation has focused primarily on butyrate-producing Firmicutes such as Roseburia intestinalis and Faecalibacterium prausnitzii, where paired CE2 and CE17 acetylmannan esterases act in tandem to fully deacetylate glucomannan and galactoglucomannan backbones, homologous CE2/CE17-containing mannan PULs are widely distributed across gut Bacteroides and related taxa (Michalak et al., 2020; Michalak et al., 2020b). In these systems, CE17-type esterases preferentially remove 2-O acetyl groups that sterically block mannanase access, while CE2-type esterases then remove 3-O, 4-O, and 6-O acetylations, thereby exposing the β-(1→4) mannosyl (or glucomannosyl) backbone to GH26/GH113 endomannanases and downstream β-mannosidases for complete depolymerization (Michalak et al., 2020; Michalak et al., 2020b; Lindstad et al., 2020).
Acemannan is an acetylated β-(1→4) glucomannan from Aloe vera, featuring a mannose-rich backbone with acetyl substitutions at positions that closely match the acetylation patterns of plant glucomannans and galacto-glucomannans used as substrates in these PUL characterization studies (Michalak et al., 2020). On this structural basis, acemannan is an excellent candidate substrate for the same CE17 + CE2 esterase pairs embedded in human gut β-mannan PULs, particularly within Bacteroides spp., Roseburia spp., and Faecalibacterium prausnitzii, which have been shown to deploy such systems on dietary β-mannans (Michalak et al., 2020; Michalak et al., 2020b; Reddy et al., 2016; Bågenholm et al., 2019).
To date, however, acemannan itself has not been used as the primary assay substrate in enzyme-level studies in Bacteroides, and no single Bacteroides carbohydrate esterase has been conclusively mapped as “the” acemannan deacetylase (Reddy et al., 2016; Déjean et al., 2020). Collectively, the best-supported mechanistic model is that CE2 and CE17 acetylmannan esterases, colocalized within β-mannan PULs and acting together with GH26/GH113 mannanases and associated β-mannosidases, form the core enzymatic machinery by which gut Bacteroides and allied commensals deacetylate and depolymerize Aloe-derived acemannan in vivo, even though this has so far been inferred from work on structurally analogous acetylated β-mannans rather than demonstrated directly on purified acemannan (Michalak et al., 2020; Michalak et al., 2020b; Lindstad et al., 2020; Reddy et al., 2016).
Keywords: Aloe arborescens; enzyme inhibition; in vitro safety; microbiological activity; scratch test.
Source of validity: Scientific
Bacteroides and Acetylated Mannans: Implications for Acemannan Metabolism
Human gut Bacteroidetes harbor specialized β-mannan polysaccharide utilization loci (PULs) that are transcriptionally induced by galactomannans, glucomannans, and related acetylated β-mannans, and typically encode surface- and periplasmic endo-β-mannanases (predominantly GH26, with occasional GH113), exo-acting β-mannosidases such as the retaining family Bs164, as well as accessory functions including α-galactosidases, SusC/SusD-like transporters, and one or more carbohydrate esterases for O-acetyl removal (Bågenholm et al., 2017; Reddy et al., 2016; Feng et al., 2022).
In Bacteroides ovatus, a defined β-mannan (galactomannan) PUL (BoManPUL/BACOVA_02088–97) is essential for growth on complex dietary mannans, with a modular enzymatic system in which a surface-exposed GH26 endomannanase (BoMan26B) initiates galactomannan cleavage at the outer membrane, and periplasmic GH26 and GH36 enzymes further depolymerize and debranch imported oligosaccharides (Bågenholm et al., 2017; Reddy et al., 2016). Heavy galactosyl substitution and O-acetylation of the mannan backbone decrease the efficiency of this system, highlighting the requirement for dedicated α-galactosidases (e.g., BoGal36A) and carbohydrate esterases within the same PUL to remove side chains and acetyl groups before complete saccharification (Reddy et al., 2016; Feng et al., 2022).
These mechanistic insights imply that structurally related acetylated mannans such as acemannan will be metabolized by Bacteroides via analogous PUL-encoded enzyme consortia, where the interplay between endo-β-mannanases, exo-mannosidases, α-galactosidases, and acetyl esterases determines both the efficiency of utilization and the pattern of oligosaccharide and short-chain fatty acid outputs in the colon (Bågenholm et al., 2017; Feng et al., 2022).
Polysaccharide Utilization Loci for Acetylated β‑Mannans in Gut Bacteroides
Polysaccharide utilization loci (PULs) for β-mannan catabolism in gut bacteria typically encode a coordinated pair of carbohydrate esterases that remove backbone acetylations prior to glycoside hydrolase attack.
In Roseburia intestinalis, detailed biochemical and structural work established a complementary esterase system in which the CE2 enzyme (RiCE2) preferentially hydrolyzes 3-O, 4-O, and 6-O acetyl groups from mannan and galacto-glucomannan backbones, whereas the CE17 acetylmannan esterase (RiCE17) is highly specific for axially oriented 2-O acetyl substituents on mannose residues in β-mannans and glucomannans, including doubly acetylated units. This division of labor is now recognized as a hallmark of CE2/CE17 pairs that are frequently colocalized within mannan-targeting PULs in prominent butyrate-producing Firmicutes such as R. intestinalis and Faecalibacterium prausnitzii.
Comparative genomics and curated PUL databases reveal that analogous CE2- and CE17-like esterase genes are also embedded in β-mannan utilization loci of multiple human gut Bacteroides and Parabacteroides species, usually in proximity to GH26/GH5 mannanases and SusC/D-like transport modules, indicating that these Bacteroidetes deploy a conserved enzymatic strategy for stepwise deacetylation and depolymerization of dietary acetylated β-mannans. This recurrent CE2/CE17 organization across phylogenetically distinct gut commensals supports the view that selective removal of 2-O versus 3/4/6-O acetyl groups is a central, conserved adaptation for efficient access to structurally complex mannan fibers in the mammalian intestine.
In vitro fermentation work on Aloe-derived polysaccharides identifies Bifidobacterium spp. as the most efficient and directly demonstrated acemannan metabolizers, with growth-kinetic and substrate-use data showing that selected Bifidobacterium strains ferment acemannan at levels comparable to commercial fructooligosaccharides and more readily than Lactobacillus spp. (Huerta-Ocampo et al., 2017; Huerta-Ocampo et al., 2018). In these systems, acemannan and Aloe whole-leaf preparations support acetate-dominant SCFA profiles and contribute to butyrate formation, indicating functionally relevant fermentation and a shift toward metabolites known to fuel colonocytes and stabilize tight junction complexes (Pogribna et al., 2008; Huerta-Ocampo et al., 2018). SCFAs such as acetate and butyrate, in turn, are well established to enhance epithelial barrier integrity and constrain excessive inflammatory signaling, aligning acemannan-driven microbial activity with a more homeostatic mucosal immune tone (Pogribna et al., 2008).
By contrast, Lactobacillus spp. and several other probiotic taxa display weaker growth on intact, high-molecular-weight acemannan, preferentially utilizing simpler carbohydrates or shorter fructans and showing only modest expansion when acemannan is the principal carbon source—a pattern consistent with limited mannanase capacity and the rheological constraints imposed by the polymer matrix (Huerta-Ocampo et al., 2017; Huerta-Ocampo et al., 2018).
CE2 and CE17 Acetyl-Mannan Esterases in Deacetylation of Glucomannans
Once acetyl groups are removed from acetylated β-mannans by carbohydrate esterases of families CE2 and CE17, the β-mannan polysaccharide utilization loci (PULs) of human gut Bacteroides deploy a coordinated set of backbone-cleaving and exo-acting hydrolases to convert the deacetylated glucomannan into fermentable sugars (Mafa et al., 2023). This system uses endo-β-mannanases from GH26 and GH113 families to attack the β-(1→4) mannan or glucomannan backbone, generating soluble manno-oligosaccharides that can be further processed in the periplasm (Gao et al., 2021; Sun et al., 2022; Peng et al., 2023). Subsequently, β-mannosidases such as Bs164 from Bacteroides salyersiae, the founding member of GH164, hydrolyze β-linked mannose residues from the non-reducing ends of these oligosaccharides to release free mannose (Armstrong et al., 2019). Together, the deacetylating activity of CE2/CE17 acetylmannan esterases and the concerted actions of GH26/GH113 endo-β-mannanases with exo-acting β-mannosidases form an integrated esterase–hydrolase cascade that enables efficient depolymerization and utilization of structurally complex, partially acetylated mannans that would otherwise be recalcitrant to digestion in the gut environment (Mafa et al., 2023; Gao et al., 2021).
Once the blocking O-acetyl groups have been removed by PUL-encoded carbohydrate esterases, β-mannan PUL systems in human gut Bacteroides deploy endo-β-mannanases from GH26 and GH113 to attack the now-accessible β-(1→4) mannan or glucomannan backbone, generating a mixture of soluble manno-oligosaccharides that can be further imported and metabolized (Couturier et al., 2022; Gharechahi et al., 2023; Peng et al., 2023). In a subsequent exo-acting step, β-mannosidases, including the GH164 enzyme Bs164 from the human gut symbiont Bacteroides salyersiae, hydrolyze terminal β-mannosidic linkages at the non-reducing ends of these oligosaccharides, releasing free mannose for central carbon metabolism (Bågenholm et al., 2019). Together, this coordinated esterase–endomannanase–β-mannosidase cascade provides an efficient route for deconstructing structurally complex, partially acetylated dietary mannans that are otherwise highly recalcitrant to host digestion, thereby expanding the glycan niche available to Bacteroides and supporting cross-feeding to other members of the gut microbiota (Couturier et al., 2022; Bågenholm et al., 2019).
Relevance to Acemannan
Acemannan is an acetylated β-(1→4) glucomannan composed primarily of O-acetylated mannosyl residues with minor glucose and galactose substitutions, a structural motif that closely resembles konjac glucomannan and positions acemannan as a plausible substrate for β-mannan utilization systems characterized in gut commensals such as Bacteroidesand Roseburia (Ramamoorthy et al., 1996; Bai et al., 2023; Michalak et al., 2020). Human fecal microbiota are able to depolymerize konjac glucomannan almost completely to manno-oligosaccharides and free mannose, indicating a rich repertoire of β-mannanases, β-mannosidases, and accessory esterases in the colon; by analogy, the same enzymatic toolkit is expected to act on acemannan’s glucomannan backbone in vivo (Matsuura et al., 1998; Nie et al., 2024). Within this context, dedicated β-mannan polysaccharide utilization loci (PULs) encode complementary CE2 and CE17 carbohydrate esterases that efficiently remove 2-O, 3-O, and 6-O acetyl groups from complex β-mannans and glucomannans, providing a mechanistic template for how O-acetyl groups on acemannan’s mannosyl residues could be stripped in the distal gut (Michalak et al., 2020; La Rosa et al., 2023).
Following deacetylation, PUL-encoded GH26 and GH113 endo-β-mannanases, together with exo-acting β-mannosidases, cleave the deacetylated glucomannan into fermentable manno-oligosaccharides and mannose, as demonstrated for Bacteroides ovatus and other gut bacteria growing on glucomannan substrates; this enzymatic paradigm strongly supports a model in which acemannan is systematically deconstructed by Bacteroides-associated β-mannan PUL machinery in the human colon (Bågenholm et al., 2019; Sun et al., 2022; Nie et al., 2024; Yu et al., 2025). Acemannan is an acetylated β-(1→4) glucomannan with O-acetylated mannosyl units and minor glucose and galactose substitutions; its backbone and acetylation pattern make it an excellent conceptual substrate for Bacteroides β-mannan PUL machinery (Ramamoorthy L. et al., 1996; Bai Y. et al., 2023).
AMB WELLNESS has developed a proprietary with a unique process isolating Acemannan from Aloe Vera Inner Gel with a high content of Acemannan ranging from 10% up to 25% measured by Nuclear Magnetic Resonance (NMR). Designed for high-end cosmetics, healthcare, and nutraceutical applications, Acetypol™ redefines efficacy, supporting skin hydration, barrier function, immune modulation, and gut health, positioning AMB WELLNESS at the forefront of innovation where scientific precision, purity, and performance meet unmatched effectiveness.Acetypol™ offers a more reliable and scientifically controlled alternative to conventional Aloe products, enabling formulators to achieve reproducible results by treating acetylation, purity, and molecular weight as key quality parameters rather than variable outcomes of processing.Acetypol™ offers a more reliable and scientifically controlled alternative to conventional Aloe products, enabling formulators to achieve reproducible results by treating acetylation, purity, and molecular weight as key quality parameters rather than variable outcomes of processing.Acetypol™ is a highly standardized Aloe vera–derived ingredient enriched to 15–20% acemannan with a high degree of acetylation (DA), controlled molecular weight, and high purity.
Share it on:
Latest News

ALOE SUNBURN CARE
It is now believed that chronic exposure to sunlight is detrimental to human skin. In mild cases, this damage may cause increased creasing and wrinkling of the dermis, irregular thickening, and thinning, yellowing and drying: in short, “premature aging.” More extreme acute exposure to sunlight often causes acute erythema and inflammation (commonly referred to as sunburn).

ALOE VERA ACNE SKIN CARE
Acne is a common skin disease, especially in teenagers. However, adult acne is not rare either. Acne usually shows when the nature of the skin is changed either because of bacterial colonization of the skin surface or androgen-induced changes in the sebaceous follicles.

SLOW DOWN THE APPEARANCE OF WRINKLES WITH ALOE VERA
The aging process is a challenging human experience common to everyone, and the desire to look young prevails in most of us. Aloe Vera offers vast amounts of information on the benefits of antiaging activity and skin care, helping in the exploration of possibilities of developing new anti-aging cosmeceuticals with natural approaches for anti-wrinkle slow-down applications.